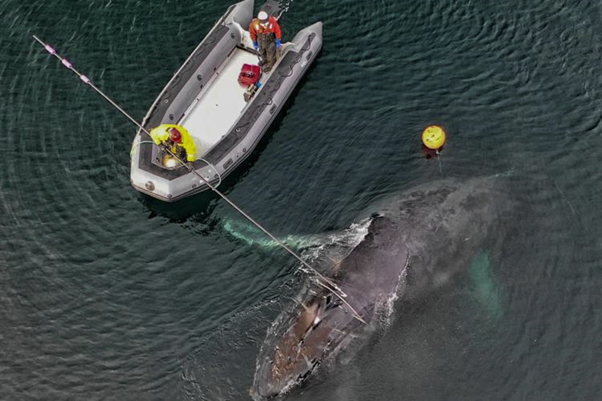
Zoop Gone Missing: A Whale’s Dinner Dilemma

Dawson Mohney, TOPAZ/JASPER HS Intern, Pacific High School Graduate

My name is Dawson Mohney, I am a high school intern for the 2025 TOPAZ/JASPER team this field season. I first heard about the TOPAZ/JASPER internship from my friend Jonah Lewis, a previous intern from the 2023 field season. Coincidentally, Jonah and I both graduated this year from Pacific High School here on the coast—small world. I have called Port Orford my home for most of my life, and in recent years I discovered that a gray whale research project has been happening in my own backyard. Growing up less than a mile from the Oregon Coast, I’ve spent a lot of time looking out into the water. I always liked how, no matter what happened in my life, the ocean was always there. This interest is what encouraged me to apply for the internship with the hope of discovering more about the ocean, a substantial part of my home and family.
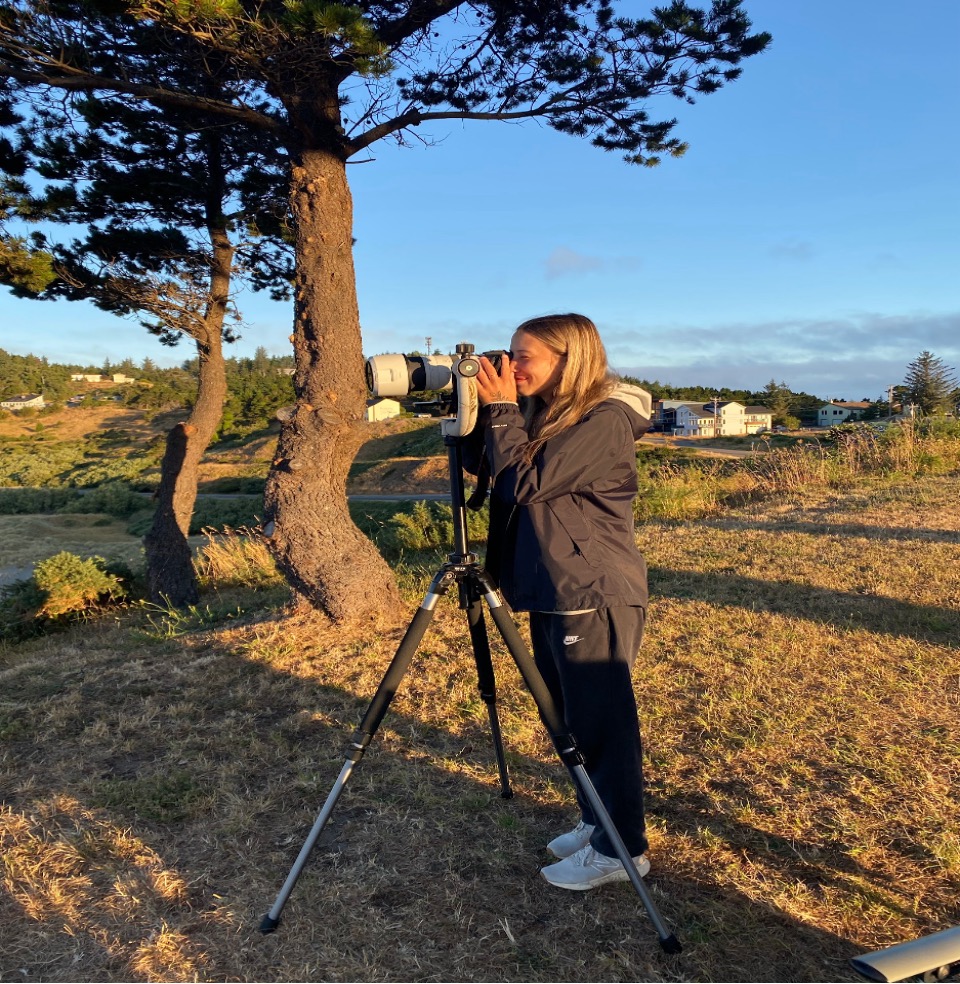
Fig 1: Picture fellow intern Maddie took of me (Dawson) during our trip to Natural Bridges.

A critical part of this project is understanding not only the magnificent gray whales but also the much less apparent zooplankton–after all, the whales need to eat a lot of zooplankton! Many different species of zooplankton—“zoop” for short—call the Oregon coast home. Each day, as we kayak to our 12 sample stations within the gray whale feeding grounds of Mill Rocks and Tichenor’s Cove, I find myself wondering which species of zoop I’ll get to identify later under the microscope.

Throughout the duration of this internship, our team has met to discuss a few research papers published by GEMM Lab members, including research produced from the TOPAZ/JASPER projects. Recently, I read, “Do Gray Whales Count Calories? Comparing Energetic Values of Gray Whale Prey Across Two Different Feeding Grounds in the Eastern North Pacific,” by Hildebrand et al. who describe the caloric content of different zooplankton species. Before reading this paper, I didn’t realize whale prey could vary in nutritional value – much like food for humans. This paper made it clear that each of the different species of zooplankton is just as important as the last, but consuming more of the higher caloric species such as the Neomysis rayii or the Dungeness crab larvae would certainly be a welcome meal. Seeing these “healthy” meals in the area makes me hopeful for the whales.
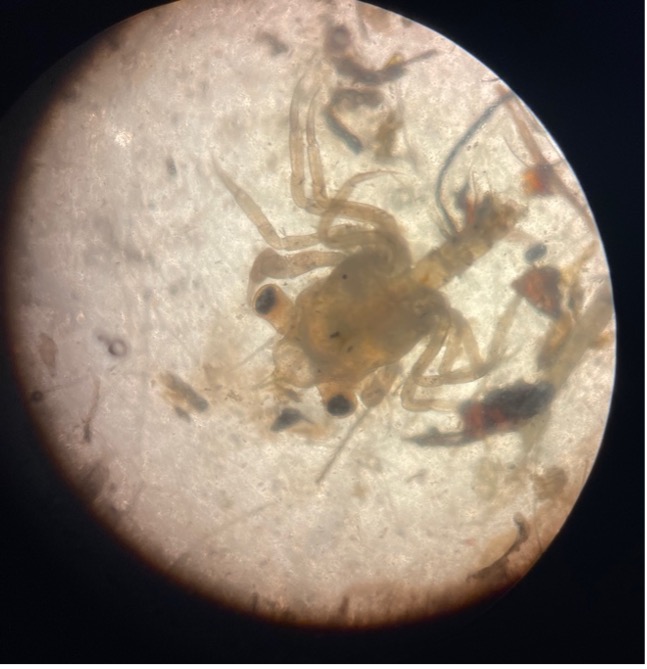
Fig 2: Image of a crab larvae in their megalopae stage.

From reading previous blog posts, the foraging habits of the whales this season appear to be unusual. In prior TOPAZ/JASPER field seasons, gray whales have often been tracked foraging near or around our Mill Rocks and Tichenor Cove study sites. This season, we haven’t tracked a single whale in Mill Rocks and only two in Tichenor Cove. Could there just not be enough good zoop?

Along with this lack of whales, there does seem to be a lack of these “high calorie zoop species”. Our team has most frequently collected samples primarily comprising of Atylus tridens, a lower calorie prey type. In fact, during one of our earlier kayak training days this field season we collected 2,019 individual A. tridens. However, since this day we have collected sparse amounts of zooplankton in our samples, ranging from zero to 121 in a given sample. Our total zoop count thus far is 2,524 zooplankton, a third of the total zooplankton collected last field season.
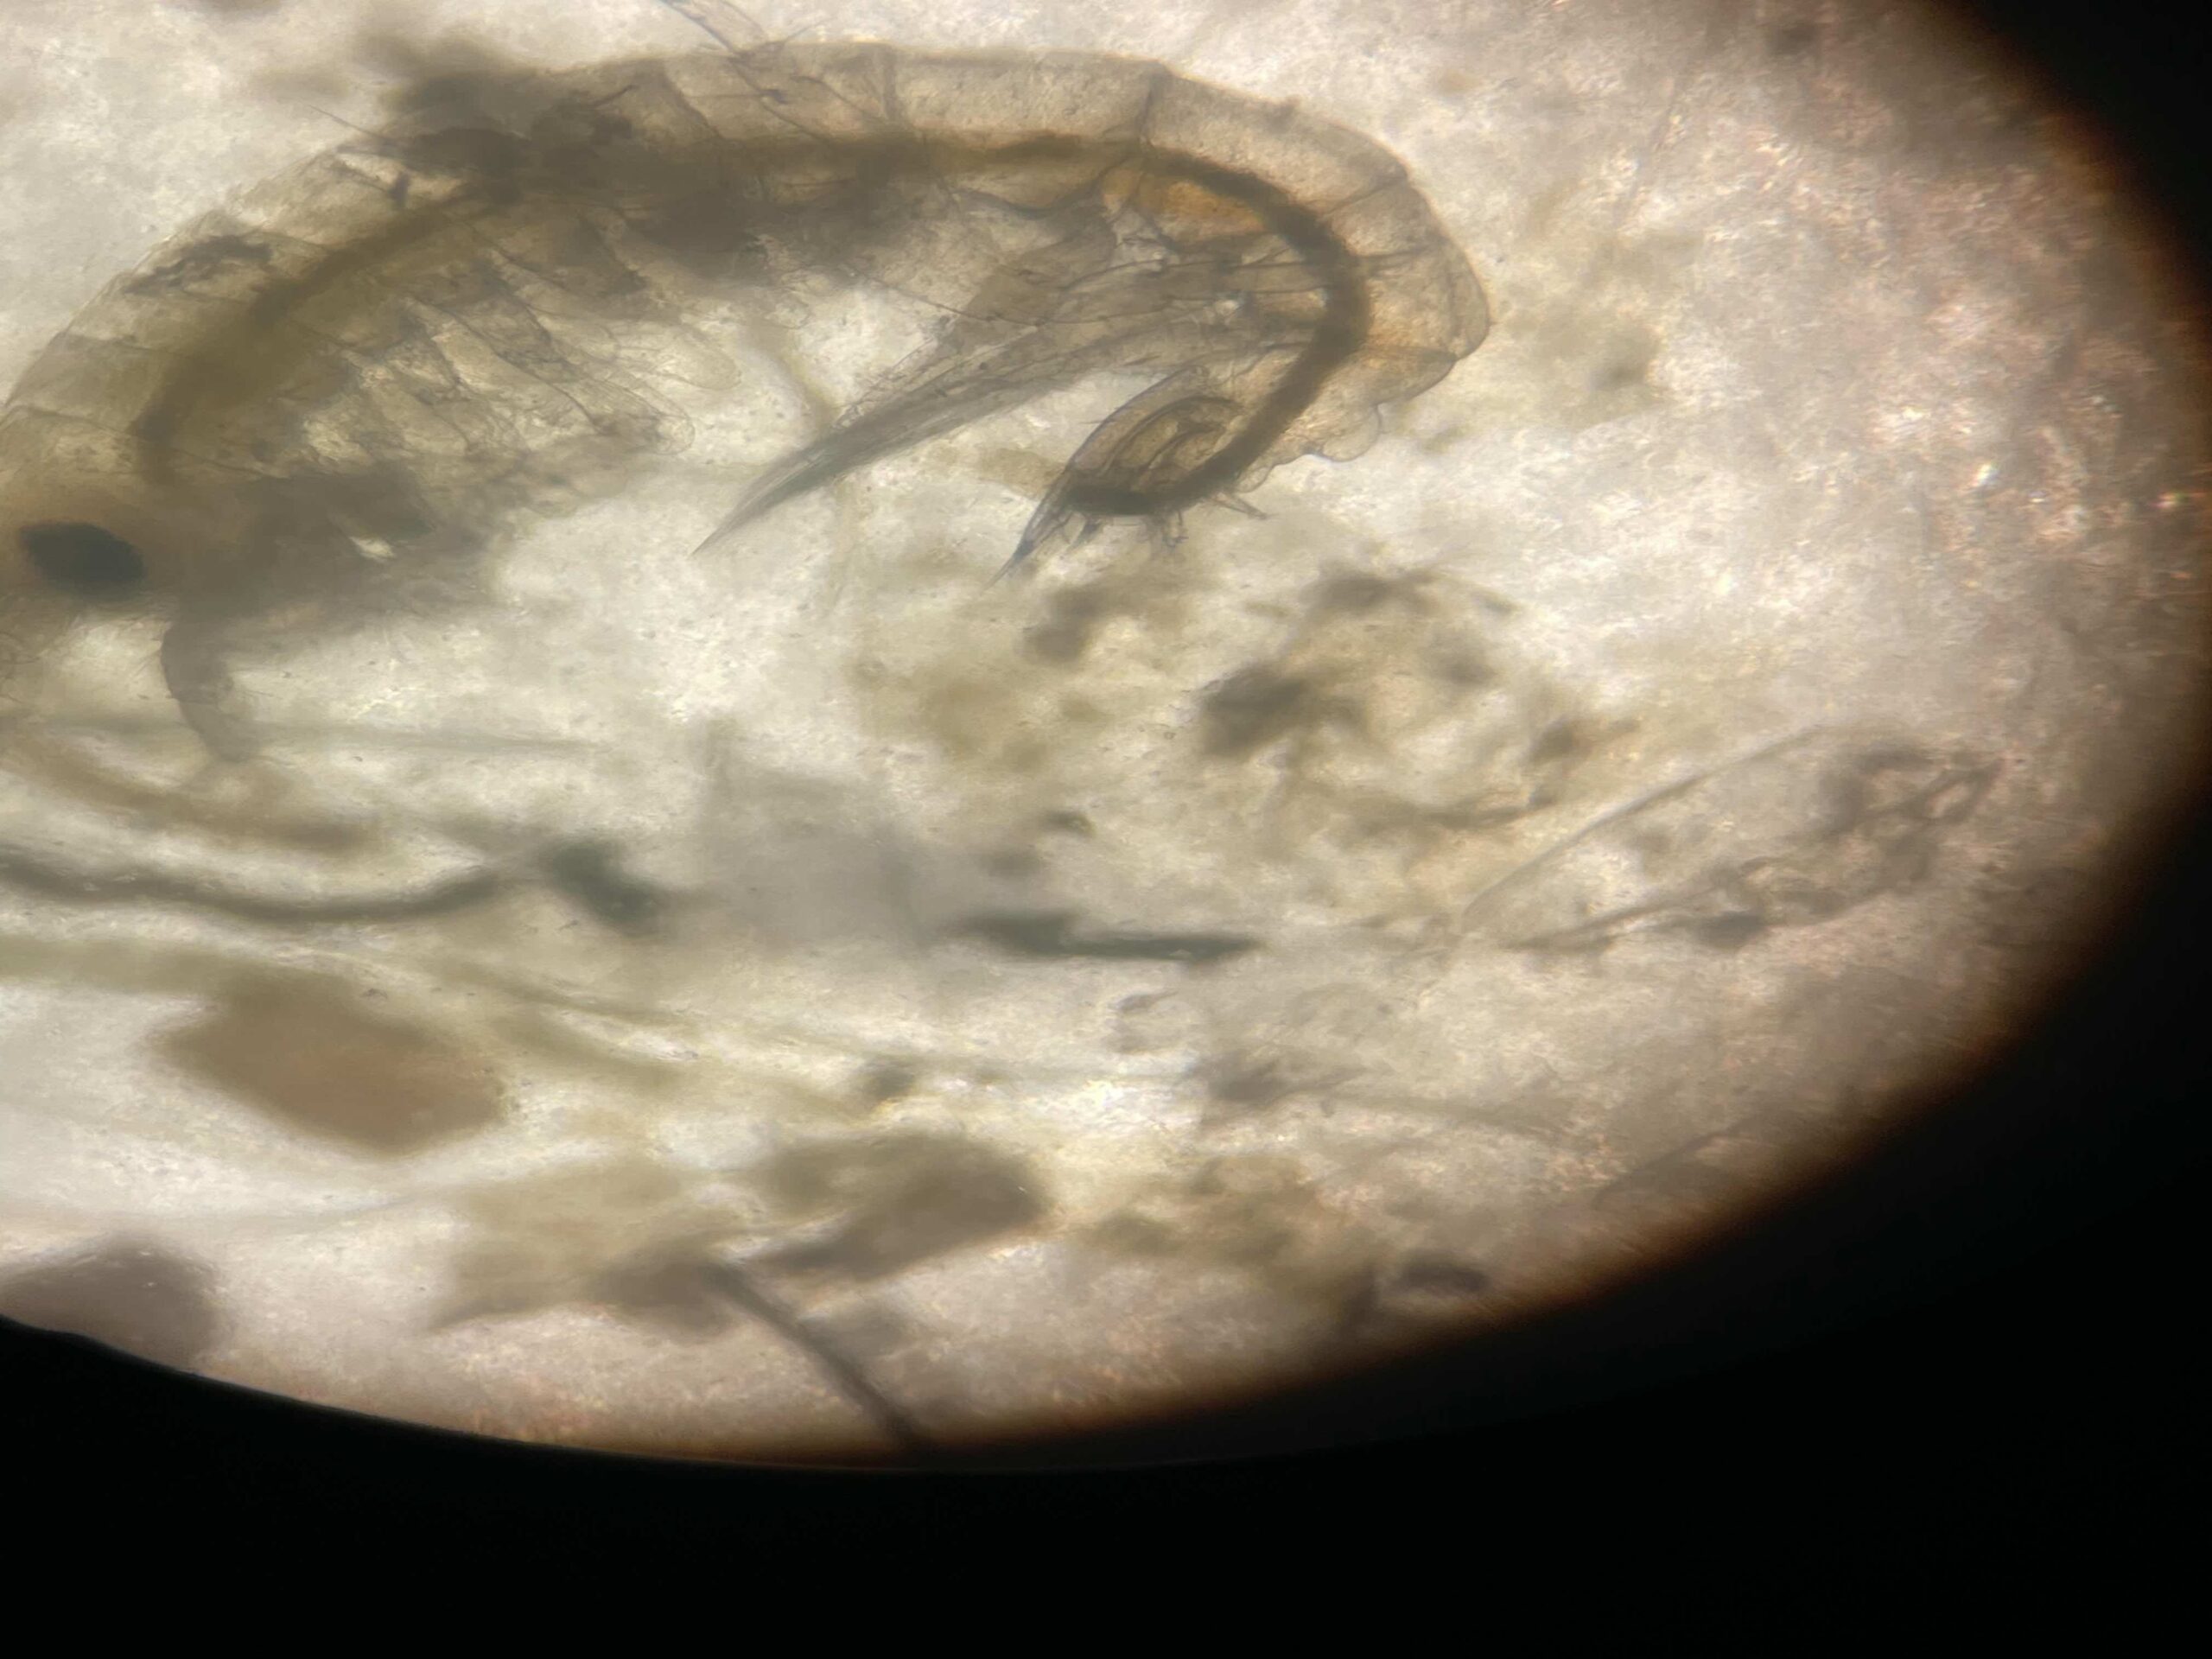
Fig 3: Image of an Atylus tridens under a microscope.

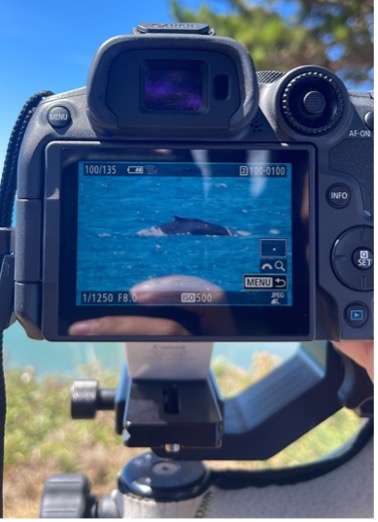
As for whale presence, we have been observing many whales blows near Hell’s Gate as mentioned in last week’s blog written by fellow intern Miranda Fowles. From our cliff site, it has been difficult to know whether these are gray whales or a different kind of whale, leading us to venture out to the Heads to get a better look. The persistence of whales in this area is certainly unusual, and perhaps it can be explained by a larger amount of higher calorie zooplankton species in the Hell’s Gate area.
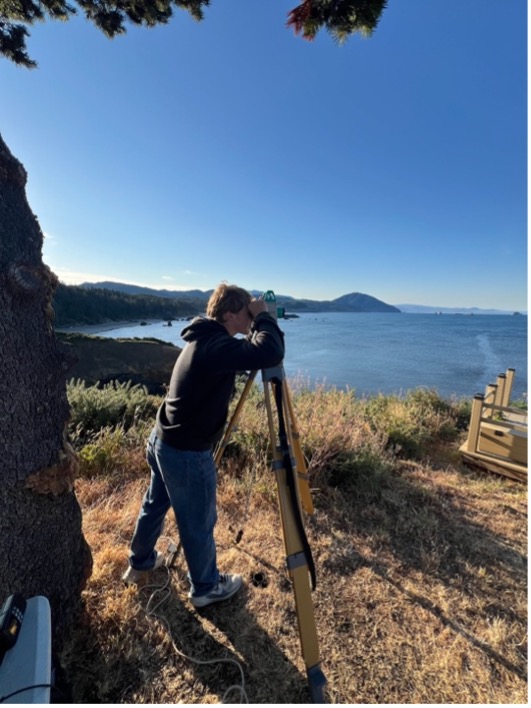
Fig 4: Dawson tracking blows by Hell’s Gate with the theodolite.

Being part of the TOPAZ/JASPER project, I have become exposed to what the true meaning is behind “fieldwork,” including learning how to be flexible and adapt to new challenges every day. What I have most enjoyed is the team’s ability to overcome any new hurdle together as a unit.  My dad often says, “You learn something new every day,” and this internship couldn’t embody this quote more. In just these 5 weeks, it almost feels like my head is now a couple sizes bigger.

Before this experience, I never thought much about how one might track a whale or how different microscopic species could have such a profound impact on a whale’s decision to forage. Now I feel I understand just how important these less than obvious factors are and the effort which goes behind understanding these relationships. I can only hope future opportunities teach me as much as joining the TOPAZ/JASPER legacy has—it’s an experience that, even just a few days into the 2025 field season, I knew would be hard to match.
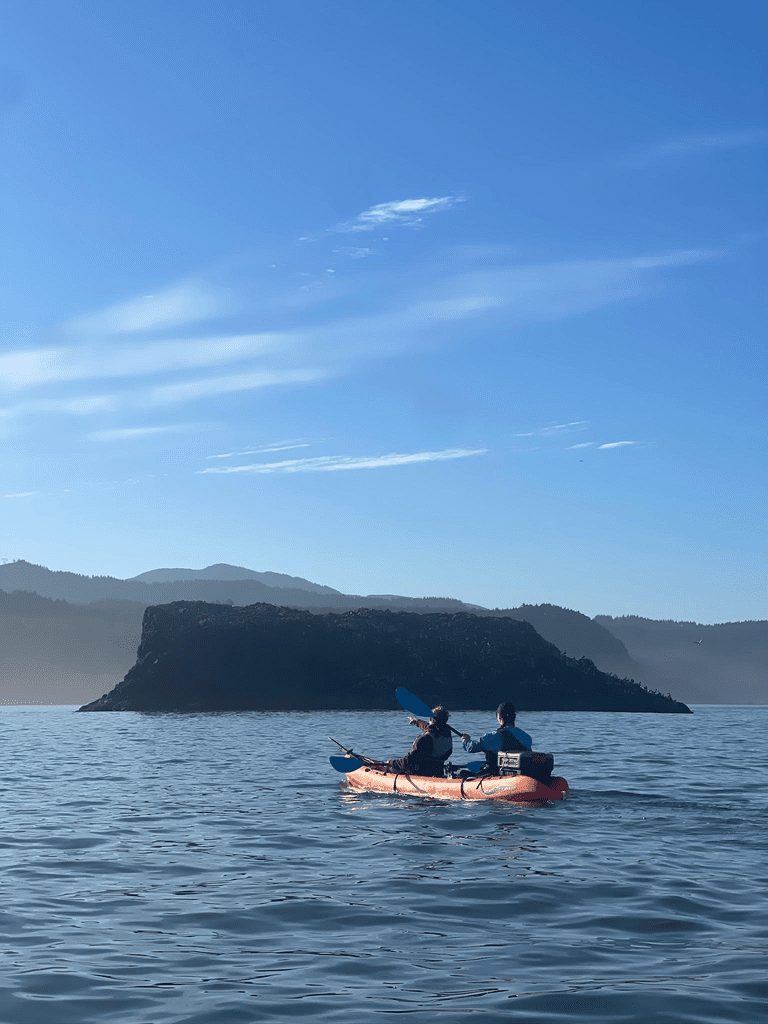
Fig 4: Dawson (navigator) and Miranda (sampler) during kayak training on their way to Mill Rocks.

Hildebrand, L., Bernard, K. S., & Torres, L. G. (2021). Do Gray Whales Count Calories? Comparing Energetic Values of Gray Whale Prey Across Two Different Feeding Grounds in the Eastern North Pacific. Frontiers in Marine Science, 8, 683634. https://doi.org/10.3389/fmars.2021.683634
Whales Off Course: Theodolite Tracking in an Unpredicted Area

Miranda Fowles, GEMM Lab TOPAZ/JASPER Intern, OSU Fisheries and Wildlife Undergraduate

Hello! My name is Miranda Fowles, and I am the OSU intern for the 2025 TOPAZ/JASPER project this summer! I recently earned my bachelor’s degree – almost, I have one more term, but I walked at commencement in June – from Oregon State University in Fisheries, Wildlife and Conservation Sciences and a minor in Spanish. My interest in whales began at a young age during a visit to SeaWorld. While I didn’t enjoy the killer whale shows for their entertainment aspect, this exposure allowed me to see a whale for the first time. From then on, I knew I wanted to contribute to understanding more about these animals, even if I wasn’t always sure how to make that happen. My decision to pursue Fisheries and Wildlife sciences was set from the beginning, however I wondered if there were actually opportunities to study whales.

Last summer, I was a MACO intern and stayed at the Hatfield Marine Science Center where I met last year’s TOPAZ/JASPER REU student, Sophia Kormann, and she raved all about her experience, so I just had to apply for this year’s internship! I remember feeling so nervous for the interview, but Dr. Leigh Torres and Celest Sorrentino’s kindness and inspiration quickly put me to ease. When I found out I was offered the position, I was just more excited than I’d ever been!

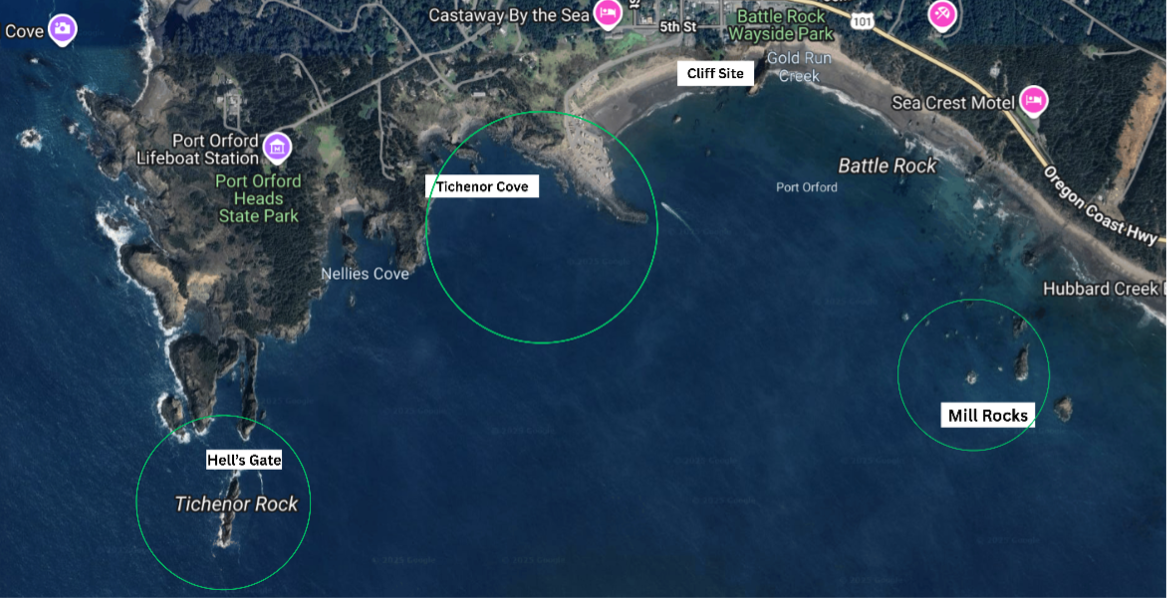
My day-to-day life as a TOPAZ/JASPER intern here at the Port Orford Field Station looks one of two ways: either on the kayak or the cliff site. When we are ocean kayaking, we go to our 12 sampling sites in the Mill Rocks and Tichenor Cove study areas (Fig. 1), where we collect zooplankton samples (Fig. 2) and oceanographic data with our RBR (an oceanographic instrument), as well as GoPro footage. When on the cliff site, we keep our eyes peeled for any whales to take pictures of them and mark their location in the water with a theodolite.

Fig. 1: Map of our study sites (Tichenor Cove and Mill Rocks) and where we have been seeing gray whales (Hell’s Gate) circled in green, and our Cliff Site.
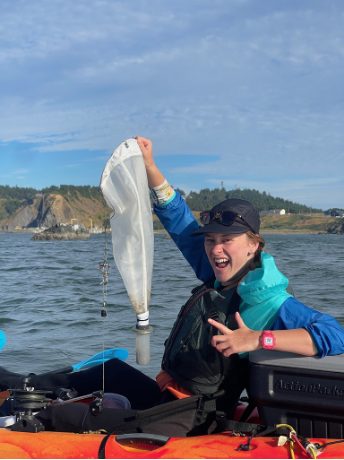
Fig. 2: Miranda Fowles out on the kayak pointing at her zooplankton samples.

A theodolite is an instrument that is used for mapping and engineering; in our case it is used to track where a gray whale blows and surfaces (For more info, please see this blog by previous intern Jonah Lewis). Each time a whale surfaces, we use the theodolite to create a point in space that marks its location. Once we have multiple points, we can draw lines between each point to establish the track of the whale. These tracklines can then be used to make assumptions of the whales’ behavior. For example, if the trackline is straight, and the individual is moving at a consistent speed and direction, we can assume the whale is transiting. Whereas if the trackline is going back and forth in one small area, the whale is likely searching or foraging for food (Hildebrand et al., 2022).

In last week’s blog my peer Nautika Brown showed how photo ID is a critical part in our field methods. When theodolite tracking, we assign a number with each new individual whale observation. If the whale is close enough, we also capture photographs of the whale (Fig. 3) and match it up to its given number, allowing us to link the trackline to an individual whale so we can understand more about individual behavior. Documenting individual specific behavior is important because previous research has shown that age, size and the individual ID of a whale can all influence different foraging tactic use (Bird et al., 2024). Therefore, each season as we collect more and more data, we establish a repertoire of recurring or new behaviors to sieve for trends and patterns.

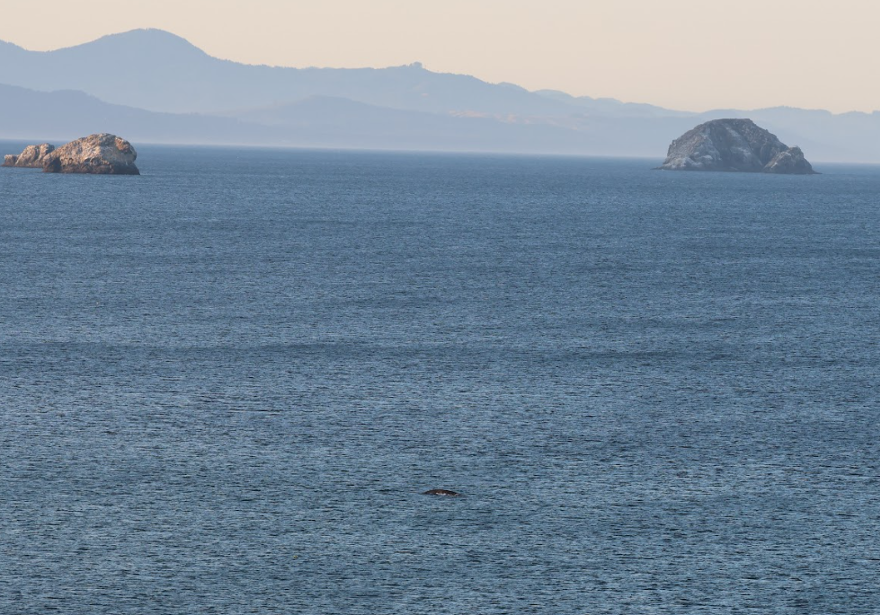
Fig. 3: Photo of a gray whale surfacing captured from our cliff site.

I find animal behavior to be an integral role in many ecological studies, and I am intrigued to explore this topic more. As marine mammals that spend most of their time underwater, cetaceans are quite an inconspicuous species to study (Bird et al., 2024), but by studying their ecology through photo ID and theodolite tracking we get insight into who they are, how they behave, and where they go.

Up until this point in the season, we have theodolite tracked gray whales for 12 hours and 3 minutes (woohoo). Interestingly, most of these tracks of whales have been near an area called “Hell’s Gate”, which is located around large rocks toward the far west of our study site (Figs. 2 and 4). We can assume, but cannot be sure, that the whales are feeding here because they spend so much time in the area, and return day after day. According to Dr. Torres, the consistent use of this area near Hell’s Gate by gray whales is unusual. In the prior 10 years of the TOPAZ project, few whales have been tracked foraging in this area near Hell’s Gate, but rather most whales have foraged in the Mill Rocks and Tichenor Cove areas. It is interesting to think about why the whales are behaving differently this year. Maybe this is due to variations in prey availability at these different sites. In recent years, Port Orford has been affected by a surge in purple sea urchin density, which have overgrazed the once prominent kelp forests here. A high urchin density decreases the kelp condition, which then leads to less habitat for zooplankton, creating a decline in prey availability for gray whales (Hildebrand et al., 2024). Upon reflection of my time on the kayak, I have noticed minimal kelp and low zooplankton abundance when conducting our zooplankton drops in our Mill Rocks and Tichenor Cove study sites. Additionally, I have also noticed many purple sea urchins in our GoPro videos. With the effects of this trophic cascade in mind, not observing any gray whales in our traditional study sites is understandable. With these gray whales more commonly seen near Hell’s Gate this year, I am curious to know what prey is attracting them there. Perhaps it is a different type of prey species or one that is high in caloric value than what is in the Mill Rocks and Tichenor Cove areas.

Fig. 4: Intern Nautika Brown looking at Hell’s Gate through the binoculars. Hell’s Gate is the passage between the two large boulders in the distance.

From actively observing whales and learning from my mentor, Celest, I have started to understand that behavior is a critical piece to any form of studying gray whales (and all species). By integrating photo-ID and theodolite tracking, we can learn so much about whale behavior, from where they eat, who is spending time where, and how they may adjust their behavior in response to a changing environment. The TOPAZ/JASPER internship has allowed me to truly comprehend what field research is like, how studying the behaviors of an individual is important, and how detail and patience are extremely necessary when collecting data. As this summer is continuing, I wonder if we will continue to see gray whales primarily feeding in the Hell’s Gate area, or if we will start to observe them more in the Mill Rocks and Tichenor Cove sites like previous years. The thrill of seeing gray whales is unlike any other, and I am so ready to see more whales this season!

References:

Bird, C. N., Pirotta, E., New, L., Bierlich, K. C., Donnelly, M., Hildebrand, L., Fernandez Ajó, A., & Torres, L. G. (2024). Growing into it: Evidence of an ontogenetic shift in grey whale use of foraging tactics. Animal Behaviour, 214, 121–135. https://doi.org/10.1016/j.anbehav.2024.06.004

Hildebrand, L., Derville, S., Hildebrand, I., & Torres, L. G. (2024). Exploring indirect effects of a classic trophic cascade between urchins and kelp on zooplankton and whales. Scientific Reports, 14(1), 9815. https://doi.org/10.1038/s41598-024-59964-x

Hildebrand, L, Sullivan, F. A., Orben, R. A., Derville. S., Torres L. G. (2022) Trade-offs in prey quantity and quality in gray whale foraging. Mar Ecol Prog Ser 695:189-201 https://doi-org.oregonstate.idm.oclc.org/10.3354/meps14115

A Nauti(k)al Journey with Photo ID  

Nautika Brown, GEMM Lab TOPAZ/JASPER Intern, recent Lake Roosevelt high school graduate 

Hi everyone! I’m Nautika Brown, a recent graduate at Lake Roosevelt High School in a small town on the Colville Indian Reservation in Washington.  

Growing up in beautiful Eastern Washington, I spent most all my days outside and, from the time I could swim, I was in the water. When I was little, I used to wish I was a fish so I could live underwater and swim every day of my life. And since then, I have always been fascinated by all animals that could live in and around water. This very fascination is what sparked the idea of becoming a marine biologist. Animals AND water, perfect! 

(Left): Nautika holding a fish she caught back home in Buffalo Lake.
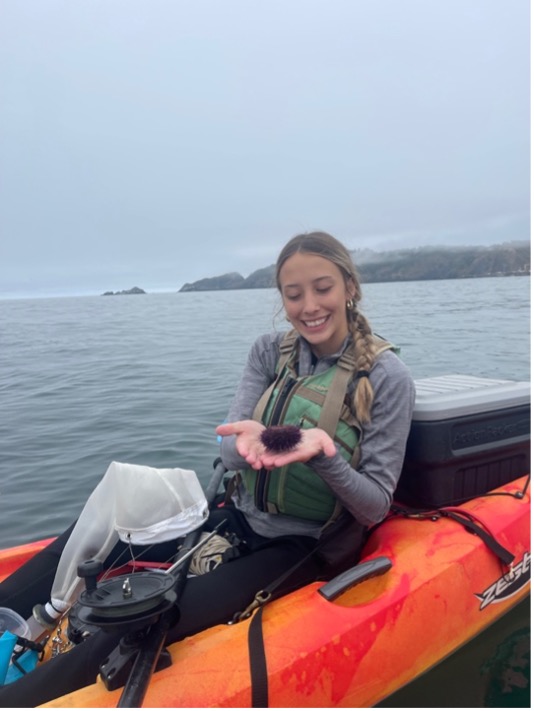
(Right) Nautika with a new type of catch (purple sea urchin) while conducting a zooplankton drop at station MR 18.

Although, as you might assume, living on a reservation surrounded by wheat fields and a few lakes, there weren’t a lot of opportunities to explore my passion. Hence, when I came across a flyer for the 2025 TOPAZ/JASPER internship just a few days before the deadline, I submitted my application as soon as I could. I was so thrilled, I couldn’t imagine getting the chance to kayak with whales on the ocean! It was all I could talk about for weeks on end. 

Since starting my internship here in Port Orford, I have learned so many new things. During our first couple weeks at the field station, we went through a few different classes and trainings, one of them being a presentation on photo identification by GEMM Lab PhD candidate Lisa Hildebrand. Prior to this presentation, I had no idea photos were so important in marine mammal science. During this presentation, I learned about the many different identifiers of a whale and how you can apply them when looking at photos to identify a specific individual. For example, Lisa’s rule of three’s: to confidently ascertain an individual’s ID, at least 3 consistent characteristics between photos must be matched. At the end of this presentation, we even played a guessing game to test our new photo ID’ing skills. (I did pretty well – not to brag or anything.) 

Now with my new photo ID skills, I was excited to capture a photo of a gray whale. On our second day of training, we did spot a whale—but thanks to my newly learned photo-ID skills, I quickly realized it wasn’t the gray whale I was expecting. When the whale first surfaced, I noticed the lack of dorsal knuckles and its distinctly darker body—clear signs it wasn’t a gray whale, but a humpback whale! While it is common to see gray whales from shore along the Oregon coast as they feed in the very nearshore habitat, humpback whales are typically found in much deeper waters, further from shore. Over the last week we have seen a humpback whale within our study site across several days—and we’re not the only ones!  When chatting with the local fisherman pre and post kayak, a few have expressed their own excitement about seeing a humpback so close to shore as well. Throughout our conversations, the question of why a humpback would be so close to shore weighed on our minds, leading me to do my own online research.  

To investigate whether these humpback sightings have been of the same individual or multiple different whales, I decided to review the photos we have captured to try and determine a match. Once I conducted a first pass of the photos, I downloaded 10 of the most clear and definite shots and compared the photos using Lisa’s rule of threes. After reviewing the photos, I noticed that the humpback whale’s dorsal hump resembled one from a previous sighting, but I couldn’t find any other distinguishing markings on its body. While I couldn’t confirm we have been observing the same humpback whale, I gained a deeper understanding of the importance of clear, high-quality photos in photo-ID work.

(Left) Nautika getting ready to take pictures of whales with camera on our cliff site. 
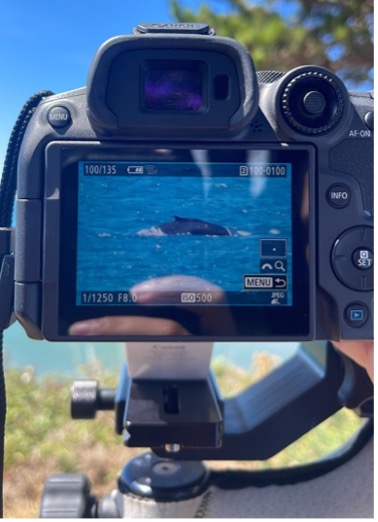
(Right) Picture of humpback whale caught on camera on our 2nd day of training

After reading a few articles about humpback whale migration through Oregon, I found a few potential reasons behind this whale’s occurrence close to the shores of Port Orford. During the summer months, humpbacks travel to colder, more nutrient-dense places to feed, often near the shelf break (where the depth of the ocean suddenly gets deeper, around 200 m). Interestingly, the shelf break near Port Orford is not far from shore, and is a known hotspot for foraging humpback whales in the summer (Derville et al. 2022).  Humpback whales filter-feed on krill and small fish, so perhaps enough prey has moved into the waters near Port Orford to attract a humpback so close to shore. Another reason for this humpback to be close to shore could be the effects of climate change. As the waters warm, food distribution changes, causing multiple species, including humpbacks, to change their feeding grounds and migration routes (read more here).  Although the humpback sightings are outside the range of our kayak zooplankton sampling stations, it would be interesting to see what prey is in the water that is keeping them around.

So far, I have learned the importance of photo identification in marine mammal science and the many ways it can be used. I’m especially grateful for Lisa’s fun and insightful presentation at the start of the season and even more surprised by how quickly I was able to put those photo-ID skills into practice. With three weeks left in the field season, I’m excited to keep building on what I’ve learned and to keep growing my skills. And speaking of building, I’m also curious to see how my “kayak muscles” are shaping up by the end of this amazing TOPAZ/JASPER internship!  

  (Left) Nautika and Celest on kayak heading Mill Rocks stations. 
(Right) Miranda and Nautika wrapping up kayak training with a celebratory team dab

Derville, S., D.R. Barlow, C. Hayslip, and L.G. Torres, Seasonal, Annual, and Decadal Distribution of Three Rorqual Whale Species Relative to Dynamic Ocean Conditions Off Oregon, USA. Frontiers in Marine Science, 2022. 9: p. 868566.

A pinch of salty, silly, and science-y: meet Team Dabwich

Celest Sorrentino, GEMM Lab Master’s student, OSU Department of Fisheries, Wildlife and Conservation Sciences, Geospatial Ecology of Marine Megafauna Lab 

As a loyal and trusted GEMM Lab blog reader, I am sure you know just what time of year it is: the beginning of the 11th annual TOPAZ/JASPER field season where we study whales and their prey while also training the next generation of scientists. The start of the season has been kicked into high tail already and we have many updates to share. Fear not, dear reader, as I am here to release you from relentlessly refreshing your inbox for the long-awaited introduction of the TOPAZ/JASPER team that is taking the project into their second decade.

But first, to appreciate the present milestone, it’s worth revisiting the legacy of those who guided us to this moment. The TOPAZ/JASPER  projects began in 2015, with PI. Dr. Leigh Torres and master’s student Florence Sullivan (2015-2018), and continued forward with Lisa Hildebrand (2018-2021), and Allison Dawn (2022-2024). Now, as a new droplet in this stream of brilliant leaders before me, I feel immense gratitude to be the master’s student leading the TOPAZ/JASPER team this summer. Having been trained by Allison Dawn with Team Protein in 2024, and full unwavering support from Leigh and each leader before me, I enter this new role with confidence and excitement for the next six gray-whale-and-zooplankton filled weeks of data collection. Now, let’s meet the young scientist interns for 2025!

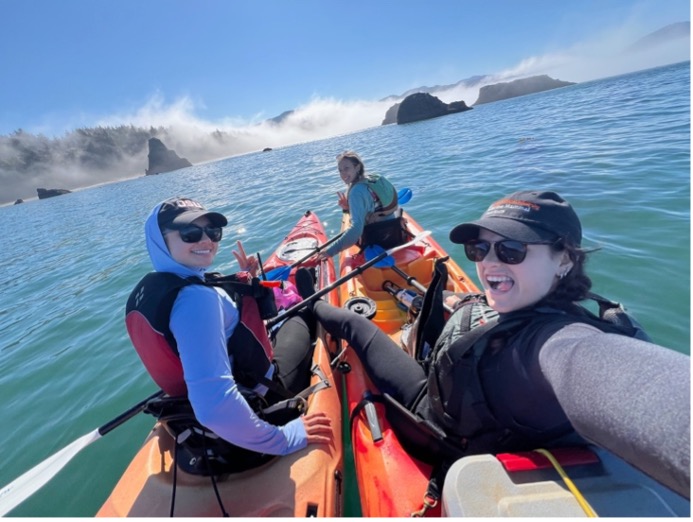
(Left picture) Maddie (right) with Nautika (top) and Celest (left) during their kayak training.
(Right picture) Photo Maddie took of a humpback in the Port Orford Bay.

Madison (Maddie) Honomichl is a senior wrapping up her last  semester of undergrad at CSU Monterrey Bay this fall to gain a degree in Marine Science. As the GEMM Lab’s REU intern this summer, Maddie began her internship in June by joining me in Newport to learn more about gray whale and pymgy blue whale mother-calf relationships. Without spoiling too much (you’ll hear more from her in her blog post in just a few weeks!) her project focuses on capturing mother-calf blow synchrony of gray and blue whales in drone footage. Now in Port Orford, her gifted talent for photography has been excellent in helping capture photos of traveling whales on the cliff.

(Left picture) Nautika finding a purple urchin after a successful zooplankton drop at our station MR 18.
(Right picture) Miranda(front) and Nautika(rear) after their first kayak training, where Nautika accidentally fell into the water but got back on the kayak in record breaking time, still in good spirits to dab!

Nautika Brown is one of our high school interns from Coulee Dam, Washington. Having just graduated, Nautika’s ambition and passion for studying wildlife lead her to apply to our TOPAZ/JASPER project and we are so happy she did. Accidentally hilarious, she has made everything from kayak training to zooplankton identification that much more enjoyable—reminding the team to have some fun while still getting the job done.

(Left picture) Dawson leading the team with the heavy theodolite stand up to the cliff.
(Right picture) The team hyper locked in on tracking a humpback whale in the bay, working together to describe the position of the whale for Dawson on the theodolite.

Dawson Mohney is our Port Orford local, having recently graduated from Pacific High School in May. Though he might not know the best spots around town, Dawson’s demeanor mirrors that of Port Orford itself: kind, welcoming, and always helpful. Always up for any task, he is the first to ask if anyone needs help with carrying equipment up to the cliff or cooking a ground beef refried beans mash for team dinner. Come fall Dawson is excited to start his first semester at Southwestern Oregon Community college.

(Left picture) Miranda enjoying an outdoor stroll of Port Orford beaches.
(Right picture) Miranda stoked on catching so many atylus tridens for her first kayak training day!

Miranda Fowles is a recent graduate at Oregon State University having completed her major in Fisheries, Wildlife, and Conservation Sciences with a minor in Spanish. Originally from Seattle, her childhood memories include kayaking with her family, so ocean kayaking has come naturally. Miranda’s genuine curiosity shines through in her eagerness to ask questions about whale life histories and their social dynamics. She’s expressed a clear passion for continuing her journey in marine science and academia.

We are now T-minus 2 days until the last of the team’s training period, and we couldn’t be more thrilled for the 4 more weeks to come. Through unexpected wildlife sightings and spontaneous team jokes, our team has only grown stronger and more connected. For all of the interns, this experience is not only their first experience with marine fieldwork, but also their longest. Training days have been both rewarding and physically strengthening; we’ve watched harbor seals lounging between Mill Rocks and tracked a particularly active humpback whale that keeps surfacing in the bay—all while developing what we now call our “ultimate kayak muscles.” By the time lunch rolls around, it feels like an ultimate power recharge, to continue forward with data processing. As any marine field scientist will tell you: there’s something deeply satisfying about coming back to shore and sinking your teeth into a handmade sandwich.

And speaking of our absolute craving for sandwiches, this team has unexpectedly brought back the 2010s dab—with such enthusiasm that it was only right to fuse “dab” with our love for chips-in-sandwiches. With this, I share with your our new, very official team name:

Team Dabwich.

With the right amount of salty, silly, and scienc-y, Team Dabwich is ready to crush the 11th TOPAZ/JASPER field season.

Team Dabwich dabbing right before a successful kayak training
ヽ(⌐_⌐ゞ)!

New GEMM Lab study indicates troubled times for PCFG gray whales

Dr. Enrico Pirotta (CREEM, University of St Andrews) and Dr. Leigh Torres (GEMM Lab, MMI, OSU)

The health of animals affects their ability to survive and reproduce, which, in turn, drives the dynamics of populations, including whether their abundance trends up or down. Thus, understanding the links between health and reproduction can help us evaluate the impact of human activities and climate change on wildlife, and effectively guide our management and conservation efforts. In long-lived species, such as whales, once a decline in population abundance is detected, it can be too late to reverse the trend, so early warning signals are needed to indicate how these populations are faring.

We worked on this complex issue in a study that was recently published in the Journal of Animal Ecology. In this paper, we developed a new statistical approach to link three key components of the health of a Pacific Coast Feeding Group (PCFG) gray whale (namely, its body size, body condition, and stress levels) to a female’s ability to give birth to a calf. We were able to inform these metrics of whale health using an eight-year dataset derived from the GRANITE project of aerial images from drones for measurements of body size and condition, and fecal samples for glucocorticoid hormone analysis as an indicator of stress. We combined these data with observations of females with or without calves throughout the PCFG range over our study period.

We found that for a female to successfully have a calf, she needs to be both large and fat, as these factors indicate if the female has enough energy stored to support reproduction that year (Fig. 1). Remarkably, we also found indication that females with particularly high stress hormone levels may not get pregnant in the first place, which is the first demonstration of a link between stress physiology and vital rates in a baleen whale, to our knowledge.

Figure 1. Taken from Pirotta et al. (2025), Fig. 5. Combined relationship of PCFG gray whale length and nutritional state (combination of body size and condition) in the previous year with calving probability, colored by whether the model estimated an individual to have calved or not at a given reproductive opportunity.

Our study’s findings are concerning given our previous research indicating that gray whales in this PCFG sub-group have been growing to shorter lengths over the last couple of decades (Pirotta et al. 2023), are thinner than animals in the broader Eastern North Pacific gray whale population (Torres et al, 2022), and show an increase in stress-related hormones when exposed to human activities (Lemos et al, 2022; Pirotta et al. 2023). Furthermore, in our recent study we also documented that there are fewer young individuals than expected for a growing or stable population (Fig. 2), which can be an indicator of a population in decline since there may not be many individuals entering the reproductive adult age groups. Altogether, our results act as early warning signals that the PCFG may be facing a possible population decline currently or in the near future.

Figure 2. Taken from Pirotta et al. (2025), Fig. 1. Age structure diagram for 139 PCFG gray whales in our dataset. Each bar represents the number of individuals of a given age in 2023, with the color indicating the proportion of individuals of that age for which age is known (vs. estimated from a minimum estimate following Pirotta, Bierlich, et al., 2024). The red line reports a smooth kernel density estimate of the distribution.

These findings are sobering news for Oregon residents and tourists who enjoy watching these whales along our coast every summer and fall. We have gotten to know many of these whales so well – like Scarlett, Equal, Clouds, Lunita, and Pacman, who you can meet on our IndividuWhale website – that we wonder how they will adapt and survive as their once reliable habitat and prey-base changes. We hope our work sparks collective and multifaceted efforts to reduce impacts on these unique PCFG whales, and that we can continue the GRANITE project for many more years to come to monitor these whales and learn from their response to change.

This work exemplifies the incredible value of long-term studies, interdisciplinary methods, and effective collaboration. Through many years of research on this gray whale group, we have collected detailed data on diverse aspects of their behavior, ecology and life history that are critical to understanding their response to disturbance and environmental change, which are both escalating in the study region. We are incredibly grateful to the following members of the PCFG Consortium for contributing sightings and calf observation data that supported this study: Jeff Jacobsen, Carrie Newell, NOAA Fisheries (Peter Mahoney and Jeff Harris), Cascadia Research Collective (Alie Perez), Department of Fisheries and Oceans, Canada (Thomas Doniol-Valcroze and Erin Foster), Mark Sawyer and Ashley Hoyland, Wendy Szaniszlo, Brian Gisborne, Era Horton.

Did you enjoy this blog? Want to learn more about marine life, research, and conservation? Subscribe to our blog and get a weekly alert when we make a new post! Just add your name into the subscribe box below!

Loading

References:

Lemos, Leila S., Joseph H. Haxel, Amy Olsen, Jonathan D. Burnett, Angela Smith, Todd E. Chandler, Sharon L. Nieukirk, Shawn E. Larson, Kathleen E. Hunt, and Leigh G. Torres. “Effects of Vessel Traffic and Ocean Noise on Gray Whale Stress Hormones.” Scientific Reports 12, no. 1 (2022): 18580. https://dx.doi.org/10.1038/s41598-022-14510-5.

Pirotta, Enrico, K. C. Bierlich, Leslie New, Lisa Hildebrand, Clara N. Bird, Alejandro Fernandez Ajó, and Leigh G. Torres. “Modeling Individual Growth Reveals Decreasing Gray Whale Body Length and Correlations with Ocean Climate Indices at Multiple Scales.” Global Change Biology 30, no. 6 (2024): e17366. https://doi.org/https://doi.org/10.1111/gcb.17366. https://onlinelibrary.wiley.com/doi/abs/10.1111/gcb.17366.

Pirotta, Enrico, Alejandro Fernandez Ajó, K. C. Bierlich, Clara N Bird, C Loren Buck, Samara M Haver, Joseph H Haxel, Lisa Hildebrand, Kathleen E Hunt, Leila S Lemos, Leslie New, and Leigh G Torres. “Assessing Variation in Faecal Glucocorticoid Concentrations in Gray Whales Exposed to Anthropogenic Stressors.” Conservation Physiology 11, no. 1 (2023). https://dx.doi.org/10.1093/conphys/coad082.

Torres, Leigh G., Clara N. Bird, Fabian Rodríguez-González, Fredrik Christiansen, Lars Bejder, Leila Lemos, Jorge Urban R, et al. “Range-Wide Comparison of Gray Whale Body Condition Reveals Contrasting Sub-Population Health Characteristics and Vulnerability to Environmental Change.” Frontiers in Marine Science 9 (2022). https://doi.org/10.3389/fmars.2022.867258. https://www.frontiersin.org/article/10.3389/fmars.2022.867258

The slow, but ever turning, cycles of science: a look under the hood of the scientific method

Dr. Clara Bird, Postdoctoral Scholar, OSU Department of Fisheries, Wildlife, and Conservation Sciences, GEMM Lab & LABIRINTO

Cycles can be found everywhere in nature and our lives. From tides and seasons to school years and art projects, we’re constantly experiencing cycles of varying scales. Spring on the Oregon coast brings several important cyclical events: more daylight, the oceanographic spring transition, and the return of our beloved gray whales – just to name a few. On my own personal scale, I’ve been thinking about the cycles we experience as scientists a lot lately, since I’ve recently transitioned out of graduate school and into my current position as a postdoctoral scholar.

Starting this new postdoc has been a bit jarring, as it’s felt like starting over. Even though I’m still working at the Marine Mammal Institute and still studying gray whales, I’ve been learning new skills, knowledge and theory, which pushes me to re-start the cycle of the scientific method, the process we follow in research (Figure 1). Broadly, we start by observing a system and asking a question about a potential pattern or event we see. We then come up with a hypothesis (or two or ten) to address our question(s). The next steps are to collect the data we need to answer our question(s) and test our hypotheses, analyze that data (i.e. run some statistical models), and draw some conclusions from the analysis results. While it seems quite linear, the process of data collection and analysis always leads to more questions than answers, and we inevitably start the cycle all over again.

Figure 1. Schematic depicting the scientific method

Throughout my scientific training I’ve gained experience in all these phases, but I’ve also learned just how many add-ons and do-overs there are in this process (Figure 2). Developing questions and hypotheses often requires a long and winding path through the literature, depending on how much you already know. These steps are often some of the first and biggest steps in graduate school. You need to learn as much as you can about the field and questions you are interested in, as this will inform what has already been done, where the knowledge gaps are, and the hypotheses you’re developing. For example, we often back up a hypothesis with references to studies that have answered our question in different systems. The learning curve is steep, and it’s important to not understate the work that goes into this phase. Early in my career, I remember hearing that “asking the good questions” is a critical skill for research. At the time that sounded like some vague, innate characteristic, and working to gain this ability felt ambiguous and overwhelming. I was absolutely wrong. Like most skills, knowing how to ask good questions is more about experience than intelligence. Here, experience is a combination of reading the literature and practice formulating questions based on the literature.

Figure 2. A more realistic version of the scientific method

Beyond this lesson, I also had to learn that what qualifies a question as “good” also depends on the funding source. In many research institutions, including those in the U.S., scientists are responsible for finding the funding to run their research projects. Funding a project includes salary for the scientists (e.g., professors, grad students, post docs), the cost of collecting and analyzing the data (e.g., travel, equipment, boat time), and the cost of publishing and sharing our findings (e.g., publication costs). The programs we solicit funding from often have their own priorities, so a big part of the research cycle is finding a funding source that is interested in the kinds of questions you want to ask and then adjusting your own questions and hypotheses to align with the funding source’s priorities and budget. The actual application includes writing a proposal where we (1) summarize all the background research justifying the novelty and value of the questions we want to ask and backing up our hypotheses and (2) describe how we plan on answering those questions. Funding is competitive and we typically apply multiple times before being successful. Furthermore, we often apply to multiple funding sources to support the same project. Since each source has its own focus, this ends up being an exercise in coming up with multiple ways to frame and justify a project.

Once we have funding (which can be years after the start of the cycle), we can finally start collecting, analyzing, and interpreting the data. But each of these steps has its own sub-cycles and complexities. Data collection can take years and involve all kinds of troubleshooting equipment issues, logistics, and methods. Depending on your question, data processing and analysis may involve developing your own method. For example, our lab asks a lot of questions about the morphology and body condition of whales. But before we could answer those questions, we first had to work out the best way to accurately measure whales from drone imagery while accounting for measurement uncertainty (read more here). This separate cycle of method development involved so many sub-projects and new software tools that Dr. KC Bierlich now leads the Marine Mammal Institute’s Center of Drone Excellence (CODEX).

Data analysis and interpretation brings us back to the literature review part of the cycle. But now we are looking for examples of how similar data have been analyzed previously and for studies to which we can compare our results. Then, after testing out different models and triple checking our analysis, we’re finally ready to share our findings. We share our results through conference presentations, publications (after the peer review cycle), outreach talks, and press releases that lead to media pieces and interviews.

In addition to the excitement of sharing our findings with the world, we’re simultaneously hyper-aware of all the caveats and limitations of our work. We’re always left with a long list of follow-up questions, thus starting the cycle again. From a zoomed-out perspective these results can form a clean, linear story. But zooming in reveals the reality of years and years of multiple overlapping cycles that have had to pass roadblocks and restart countless times. For example, after nine years for research, the GRANITE project has produced an impressive suite of results addressing questions related to Pacific Coast Feeding Group gray whale morphology, health, hormones, space use, and behavior. It took years of data collection, proposal writing, training, and multiple researchers working through their own project cycles to get here (and we’re not done).

Transitioning out of graduate school has meant expanding my scope of attention to multiple cycles running in parallel, re-starting the literature review process for new projects, and spending a lot more time in the proposal writing sub-cycle. While it’s felt overwhelming at times, I’ve also enjoyed digging into new topics and skills. It’s an interesting balance of experiencing the discomfort that comes with being a beginner while simultaneously drawing comfort from the knowledge that I’ve experienced this cycle before and know how to learn something new.

A consequence of learning the scientific process is growing accustomed to this cyclical nature. As scientists we know that it’s a slow process, that every result is just the start of a new cycle, and that future work building on a result may agree or disagree with the previous finding. But the way scientific findings are shared with the public doesn’t necessarily reflect the process. Catchy headlines and brief summaries often present findings as definitive and satisfying conclusions to a story. Behind those headlines are years of set up, data collection, analysis, and a suite of caveats that we want to dig into in the future. The results of any given study reflect our best current knowledge at that point in the cycle. By design, that knowledge will grow and change as we move forward.

Did you enjoy this blog? Want to learn more about marine life, research, and conservation? Subscribe to our blog and get a weekly alert when we make a new post! Just add your name into the subscribe box below!

Loading

The whale’s scale: Emphasizing the scale of process, not the scale of observation

By Lisa Hildebrand, PhD candidate, OSU Department of Fisheries, Wildlife, & Conservation Sciences, Geospatial Ecology of Marine Megafauna Lab

Baleen whales must navigate a seemingly featureless world to locate the resources they need to survive. The task of finding prey to feed on in the vast seascapes relies on the use of several sensory modalities that operate at different scales (Torres 2017; Figure 1). For example, baleen whale vision is believed to be rather limited, with the ability to see objects about 10-100 meters away. Yet, baleen whale somatosensory perception of oceanographic stimuli is thought to be on the order of 100-1000s kilometers. This diversity in sensory ability has led scientists to believe that whales, in fact all animals, perceive cues and make decisions at several scales. As ecologists, we endeavor to understand why and when animals are found (or not found) in certain locations as this knowledge allows us to better manage and conserve animal populations. With this information we can aim to minimize potential anthropogenic disturbance and protect important resource areas, such as foraging or nursing grounds. In order to accomplish this goal, we ourselves must conduct studies and test hypotheses at several scales (Levin 1992; Hobbs 2003). As someone who tackles spatial foraging ecology questions, I am particularly interested in understanding whale behavior and movement in the context of feeding. Since accurately measuring predator and prey distribution at the same scales can be challenging, we often resort to environmental variables to serve as proxies for prey, whereby we look for correlations between environmental variables and whales to understand and predict the distribution of our population. 

Figure 1. Schematic of hypothetical interchange of sensory modalities used by baleen whales to locate prey at variable scales. X-axis represents log distance to prey from micro (left) to macro (right). Y-axis represents the relative use of each sensory modality between 0 (no contribution) to 10 (highest contribution). Each line and color represent a different sensory modality. Figure taken and caption adapted from Torres 2017.

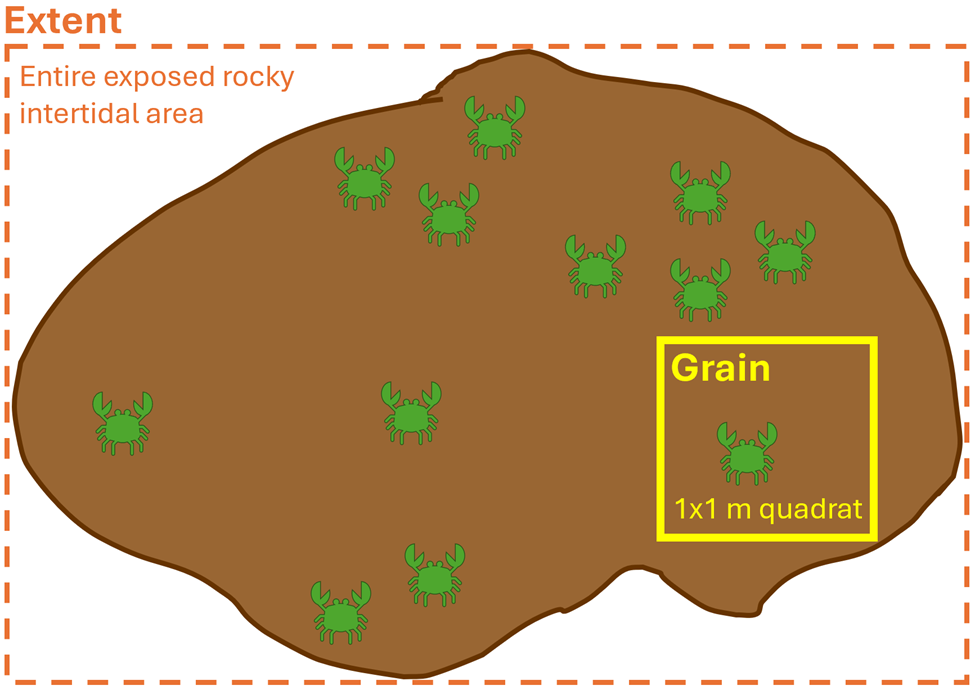
What do I mean when I use the word ‘scale’? The term scale is typically explained by two components: grain and extent (Wiens 1989). The grain is the finest resolution measured; in other words, how detailed we are measuring. The extent is the overall coverage of what we are measuring. These components can be applied to both spatial scale and temporal scale. For example, spatially, if we were using a 1×1 meter sampling quadrat to count the number of crabs on a rocky shore, then our grain would be the 1 m2 quadrat and the extent would be the entire exposed rocky intertidal area that we are surveying (Figure 2). Temporally, if we placed a temperature logger at the mouth of Yaquina Bay that took a temperature recording every minute for two years, then our grain would be one minute and the extent would be two years. So, when designing a study, it is imperative for us to decide on the spatiotemporal scales of the ecological questions we are asking and the hypotheses we are testing, as it will inform what data we need to collect. When making this decision, it is important to think about the scale at which the ecological process happens, as opposed to the scale at which we can observe the process (Levin 1992). In other words, we need to think from the perspective of our study species, as opposed to from our own human perspective. Making informed and ecologically reasonable decisions regarding the choice of scale relies on having prior knowledge of an animal’s biology, such as knowing that baleen whales might see a prey patch that is 50 meters away, but it may also somatosensorily perceive an oceanic front where zooplankton prey aggregate from 500 kilometers away.

Figure 2. Schematic of spatial scale where the extent (depicted by dashed orange box) is the entire exposed rocky intertidal area being surveyed and the grain (solid yellow box) is the 1×1 m quadrat being used to count crabs.

There is a wealth of studies that have explored space use patterns of wildlife relative to environmental variables to better understand foraging behavior. I want to share a couple from the marine mammal realm with you that I find particularly fascinating. In their 2018 study, González García and colleagues used opportunistic sightings of blue whales around the Azorean islands of Portugal and modeled their distribution patterns relative to physiographic and oceanographic variables summarized at different spatial (fine [1-10 km] and meso [10-100 km]) and temporal (daily, weekly, monthly) scales. The two variables that were most correlated with blue whale occurrence was distance from the coast and eddy kinetic energy (a measure of mesoscale variability of ocean dynamics). Both of these variables were interestingly found to be scale invariant, meaning that no matter which spatial and temporal scale was investigated, the relationship between blue whales and these two variables stayed the same; blue whale occurrence increased with increasing distance from the coast and was maximal at an eddy kinetic energy value of 0.007 cm2/s2 (Figure 3).

Figure 3. Functional response curves between presence of Azorean blue whales and distance to the coast (panel 1 on left) and eddy kinetic energy (panel 2 on right). The top row of each panel represents the low spatial scale and the bottom row represents the high spatial scale. Each column represents a different temporal scale (from left to right: daily, weekly, monthly). Note that the general shape of the relationship remains similar across all spatiotemporal scales and that the peak of the curves tend to occur at the same values for distance to coast and eddy kinetic energy across all scales. Figures taken from González García et al. 2018.

However, not all studies find scale invariant relationships. For example, Cotté and co-authors (2009) found that habitat use of Mediterranean fin whales was very much scale dependent. At a large scale (700-1,000 km and annual), fin whales were more densely aggregated during the summer in the Western Mediterranean where there was consistently colder water than in the winter. However, at a meso scale (20-100 km and weekly-monthly), fin whale densities were highest in areas where there were steep changes in temperature, as opposed to consistently cold temperatures. The authors explain that these differences in fin whale density and temperature at different scales are likely due to whale movement being driven by annually persistent prey abundance at the large scale, but at the meso scale, where prey aggregations are less predictable, the fin whales’ distribution becomes more driven by areas of physical ocean mixing.

As I investigate the environmental drivers of individual gray whale space use using our 8-year GRANITE (Gray whale Response to Ambient Noise Informed by Technology and Ecology) dataset, these studies (and many more) are at the top of my mind to interpret the patterns we are detecting. Our goal is to quantify and describe what environmental conditions (1) lead to a higher probability of a gray whale being seen in our central Oregon coast study area (~70 km) at a daily scale, and (2) influence space use patterns (activity range, residency, activity center) of different individual whales at annual scales. Our results show both consistency and variation in the environmental drivers of gray whales across these scales, leading me to deeply consider how gray whales make decisions at different points in their lives, based on information gained through various senses, to maximize their chances of capturing food. Previous work from the GEMM Lab on the relationships between gray whales and prey, at both fine (read more here) and large (read more here) scales have guided my work by providing specific hypotheses regarding environmental variables and lag times for me to test. Investigating the environmental drivers of animal space use and behavior is exciting work as it reveals that no single environmental variable determines animal distribution, but rather that multiple processes are happening concomitantly that animals respond to at different scales continually. It is only by studying animal space use patterns across spatiotemporal scales that we can begin to understand their complex decision-making patterns.

Did you enjoy this blog? Want to learn more about marine life, research, and conservation? Subscribe to our blog below and get a monthly message when we post a new blog. Just add your name and email into the subscribe box below.

Loading

References

Cotté, C., Guinet, C., Taupier-Letage, I., Mate, B., & Petiau, E. (2009). Scale-dependent habitat use by a large free-ranging predator, the Mediterranean fin whale. Deep Sea Research Part I: Oceanographic Research Papers56(5), 801-811.

González García, L., Pierce, G. J., Autret, E., & Torres-Palenzuela, J. M. (2018). Multi-scale habitat preference analyses for Azorean blue whales. PLoS One13(9), e0201786.

Hobbs, N. T. (2003). Challenges and opportunities in integrating ecological knowledge across scales. Forest Ecology and Management181(1-2), 223-238.

Levin, S. A. (1992). The problem of pattern and scale in ecology: the Robert H. MacArthur award lecture. Ecology73(6), 1943-1967.

Torres, L. G. (2017). A sense of scale: Foraging cetaceans’ use of scale‐dependent multimodal sensory systems. Marine Mammal Science33(4), 1170-1193.

Wiens, J. A. (1989). Spatial scaling in ecology. Functional ecology3(4), 385-397.

The blues are back in town: recap of the SAPPHIRE 2025 field season

By Dr. Dawn Barlow & Dr. Leigh Torres, OSU Department of Fisheries, Wildlife, and Conservation Sciences, Geospatial Ecology of Marine Megafauna Lab

As the sun set on February 16th, the R/V Star Keys pulled into Wellington Harbour, marking the end of the 2025 SAPPHIRE field season. The crew and science team returned to shore after a packed, productive, and successful three weeks at sea studying the impacts of environmental change on blue whales and krill in the South Taranaki Bight, Aotearoa New Zealand.

A blue whale comes up for air in the South Taranaki Bight.

In stark contrast to the 2024 field season, which featured dense and seemingly endless layers of gelatinous salps in the water and no krill or blue whales in the South Taranaki Bight, the 2025 field season was filled with blue whales and krill. In our three weeks aboard our research vessel Star Keys this year, we observed 66 blue whales, most of which were lunge feeding at the surface on dense patches of krill. We also collected krill for on-board respiration experiments and to be frozen to measure their lengths, weights, and caloric content. We recovered two hydrophones that recorded blue whale calls for the past year, and replaced them with two more. We collected identification photos, skin and blubber tissue samples for genetic and hormone analysis, and flew drones over almost all whales we encountered to measure body condition and morphology. We conducted water column profiles to measure the oceanography of the region, and mapped the prey field as we surveyed using a scientific echosounder.

Map of our survey effort (gray tracklines), blue whale sightings (red circles), and hydrophone locations (purple stars).

Around the world, we are currently bearing witness to environmental change. Our survey last year in 2024 was a reminder of the challenges these blue whales face to survive and thrive in an increasingly unpredictable ocean. This year was a poignant example of the vibrant marine life that exists here in the South Taranaki Bight when ocean conditions align more closely with what is expected, and of the incredible resilience of these animals as they navigate changing waters. These contrasting conditions over multiple years are key to our understanding as we study the impacts of climate change on krill and blue whales through the SAPPHIRE project.

Drone image of a blue whale coming to the surface.

The fieldwork we do to collect these data is motivated by scientific questions, management needs, and fascination with this ecosystem. But ultimately, what makes fieldwork possible and memorable is the people. We are deeply grateful for the many partners on the SAPPHIRE project. The 2025 science team was made up of Leigh Torres, Dawn Barlow, KC Bierlich, Kim Bernard (Oregon State University), Mike Ogle, and Ros Cole (Department of Conservation). The outstanding crew of the R/V Star Keys (Western Work Boats), Josh Fowden, Dave Futter, and Jordy Maiden-Drum, kept us safe, sailing, fed, and happy for three intense weeks. We are also grateful for our shore support, including our colleagues at Cornell University’s Yang Center for Conservation Bioacoustics, NIWA, the Marine Mammal Institute at Oregon State University, and the University of Auckland. Importantly, we deeply appreciate our many stakeholders who help us share, learn, and make our findings meaningful, including the Department of Conservation, the people of Aotearoa, and iwi across our study region, especially Ngāruahine who hosted us at the Rangatapu Marae for a profound hui with a powerful pōwhiri and critical wānanga of knowledge sharing.

Drone image of a blue whale mom and calf pair.

Now the next phase of the work begins. We have many terabytes of data to process, analyze, interpret, and share. We will certainly have our hands full. But while we are at our computers back in Oregon, we will be holding the memories of this field season close: The brilliant turquoise glow of a blue whale just below the surface, the sound of the deep exhalation as the whale comes up for air, and the awe of looking into a blue whale’s eye as it engulfs a dense swarm of krill; The golden sunset lighting and moon rise over Cape Farewell, and Mount Taranaki towering over the blue waters of the South Taranaki Bight; The giddy exclamations or silent awe of those of us privileged to spend time in these waters observing these animals, and the visions that linger just behind our eyelids as we fell into an exhausted sleep. We will see what the next year holds for the SAPPHIRE team and the blue whales and krill of the South Taranaki Bight.

Did you enjoy this blog? Want to learn more about marine life, research, and conservation? Subscribe to our blog and get a weekly alert when we make a new post! Just add your name into the subscribe box below!

Loading

New publication shows humpback whale distribution in the Northern California Current is related to krill swarm biomass, energetic density, and species composition

By Rachel Kaplan, PhD candidate, Oregon State University College of Earth, Ocean, and Atmospheric Sciences and Department of Fisheries, Wildlife, and Conservation Sciences, Geospatial Ecology of Marine Megafauna Lab

What does a whale look for at mealtime? Is it a lot of food, its quality, or the type of food? An improved understanding of what makes krill swarms, an important prey item, appetizing for humpback whales can help us anticipate where and when we will see them in our ocean backyard, the Northern California Current (NCC) foraging grounds. In a new paper, we found that humpback whale presence in the NCC is tied to several different metrics of krill swarm quality and quantity, particularly species composition (what types of krill are in the swarm), energetic density (the caloric richness of the average mouthful), and biomass (how much krill is in the swarm). Interestingly, relationships between humpback whales and these krill swarm quality metrics are variable in time and space, dependent on whether the whale is foraging on or off the continental shelf and if it is early or late in the foraging season.

This study required a special, fine-scale dataset of simultaneous observations of krill and whales at sea. While GEMM Lab members conducted marine mammal surveys, we simultaneously observed the prey that whales had access to, using active acoustics (essentially a fancy fish finder) to profile the water column and net tows to collect krill. When we put all these data streams together, we found that increases in biomass, energetic density, and the amount of a particular species, Thysanoessa spinifera, in a krill swarm were positively related to humpback whale presence. These results suggest that humpback whales balance multiple prey quality factors to select feeding areas that offer both plentiful and high-quality krill.

Figure 1. Top photo: Marine mammal observers Clara Bird (left) and Dawn Barlow (right) collect humpback whale distribution data. Bottom photo: At the same time, Talia Davis (left) and Rachel Kaplan (right) collect krill samples.

Species composition

Euphausia pacifica and T. spinifera are the two most common krill species in the NCC region, and other research has shown that many krill foragers, including blue whales, seabirds, and fish, preferentially consume T. spinifera. Although this pickiness is well-warranted – individual T. spinifera tend to be larger than E. pacifica and much higher in calories during the late foraging season – targeting this juicy prey item could place humpback whales in competition with these other species, which may make it harder for them to find a square meal. Nevertheless, we found positive relationships between the proportion of T. spinifera in a krill swarm and humpback whale presence, suggesting humpback whales do in fact preferentially prey upon T. spinifera, particularly during the late foraging season (about July-November).

Energetic density

Humpback whales’ preference for T. spinifera during the late foraging season may be due to its higher caloric content. Although the two krill species offer a similar number of calories early in the foraging season,we found that the energetic density of T. spinifera was elevated during the late foraging season, after productive upwelling conditions have revved up the food web over several months. Krill swarm energetic density had a positive effect on humpback whale occurrence, particularly in the late season when T. spinifera and E. pacifica have significantly different caloric contents. Interestingly, this positive relationship was not present onshore during the early season, when the two krill species have similar caloric contents.

Figure 2. In terms of caloric content, Thysanoessa spinifera krill like this one are the winners in the NCC region! They pack on the milligrams through the productive summer season, making them advantageous prey for hungry whales.

Humpback whales also target forage fish on the continental shelf that have higher energetic densities than krill, indicating that whales may selectively forage on fish – even though it is more energetically expensive to capture them. Variation in seasonal and spatial relationships with krill swarm energetic density may explain why humpback whales prey-switch, selecting prey based on availability and quality. As flexible foragers, humpback whales can consistently target higher-quality swarms that offer more energy per lunge.

Biomass

Biomass, or the total amount of krill in a swarm, was the single best predictor of humpback whale presence that we tested. This result emphasizes the importance of large krill swarms in explaining where humpback whales forage. We found that krill swarm biomass tended to be higher offshore, where swarms were also located deeper in the water column. During the late season offshore, krill quality (elevated due to higher late season caloric contents) together with quantity (higher offshore biomass) may make these offshore swarms the most favorable for foraging whales, despite being deeper.

Figure 3. When humpback whales “fluke,” as seen in this picture, it may indicate the beginning of a foraging dive to capture prey.

Future food webs

Environmental conditions are changing in the NCC, with events like marine heatwaves and strong El Niño events shifting food webs. E. pacifica and T. spinifera may respond to climate change differently based on their life history strategies. Distributional shifts, such as the disappearance of T. spinifera from the NCC during the 2014–2015 “Blob” marine heatwave that transformed the northeast Pacific Ocean, could diminish or entirely remove this key prey item. As a result of such climate and environmental changes, humpback whales may encounter lower quality prey and/or shifts in prey distribution that could make it harder for them to find a meal. In changing oceans, better understanding krill prey quality for humpback whales will shape improved tools for conservation management.

Loading

References

Chenoweth, E., Boswell, K., Friedlaender, A., McPhee, M., Burrows, J., Heintz, R., and Straley, J. 2021. Confronting assumptions about prey selection by lunge‐feeding whales using a process‐based model. Funct. Ecol., 35.

Croll, D., Marinovic, B., Benson, S., Chavez, F., Black, N., Ternullo, R., and Tershy, B. 2005. From wind to whales: trophic links in a coastal upwelling system. Mar. Ecol. Prog. Ser., 289: 117–130.

Derville, S., Buell, T. V., Corbett, K. C., Hayslip, C., and Torres, L. G. 2023. Exposure of whales to entanglement risk in Dungeness crab fishing gear in Oregon, USA, reveals distinctive spatio-temporal and climatic patterns. Biol. Conserv., 281: 109989.

Fiedler, P. C., Reilly, S. B., Hewitt, R. P., Demer, D., Philbrick, V. A., Smith, S., Armstrong, W., et al. 1998. Blue whale habitat and prey in the California Channel Islands. Deep Sea Res. Part II, 45: 1781–1801.

Fisher, J. L., Menkel, J., Copeman, L., Shaw, C. T., Feinberg, L. R., and Peterson, W. T. 2020. Comparison of condition metrics and lipid content between Euphausia pacifica and Thysanoessa spinifera in the northern California Current, USA. Prog. Oceanogr., 188.

Murdoch, W. W. 1969. Switching in General Predators: Experiments on Predator Specificity and Stability of Prey Populations. Ecol. Monog., 39: 335–354.

Nickels, C. F., Sala, L. M., and Ohman, M. D. 2018. The morphology of euphausiid mandibles used to assess selective predation by blue whales in the southern sector of the California Current System. J. Crustacean Biol., 38: 563–573.

Price, S. E., Savoca, M. S., Kumar, M., Czapanskiy, M. F., McDermott, D., Litvin, S. Y., Cade, D. E., et al. 2024. Energy densities of key prey species in the California Current Ecosystem. Front. Mar. Sci., 10: 1345525.

Robertson, R. R., and Bjorkstedt, E. P. 2020. Climate-driven variability in Euphausia pacifica size distributions off northern California. Prog. Oceanogr., 188.

Santora, J. A., Mantua, N. J., Schroeder, I. D., Field, J. C., Hazen, E. L., Bograd, S. J., Sydeman, W. J., et al. 2020. Habitat compression and ecosystem shifts as potential links between marine heatwave and record whale entanglements. Nat Commun, 11: 536.

Spitz, J., Trites, A. W., Becquet, V., Brind’Amour, A., Cherel, Y., Galois, R., and Ridoux, V. 2012. Cost of Living Dictates what Whales, Dolphins and Porpoises Eat: The Importance of Prey Quality on Predator Foraging Strategies. PLoS ONE, 7: e50096.

Tanasichuk, R. 1998a. Interannual variations in the population biology and productivity of Thysanoessa spinifera in Barkley Sound, Canada, with special reference to the 1992 and 1993 warm ocean years. Mar. Ecol. Prog. Ser., 173: 181–195.

Videsen, S. K. A., Simon, M., Christiansen, F., Friedlaender, A., Goldbogen, J., Malte, H., Segre, P., et al. 2023. Cheap gulp foraging of a giga-predator enables efficient exploitation of sparse prey. Sci. Adv., 9: eade3889.

Weber, E. D., Auth, T. D., Baumann-Pickering, S., Baumgartner, T. R., Bjorkstedt, E. P., Bograd, S. J., Burke, B. J., et al. 2021. State of the California Current 2019–2020: Back to the Future With Marine Heatwaves? Front. Mar. Sci., 8.


Are Most Whale Entanglements “Out of Sight, Out of Mind?”

By Lindsay Wickman, Postdoctoral Scholar, Oregon State University Department of Fisheries, Wildlife, and Conservation Sciences, Geospatial Ecology of Marine Megafauna Lab

Earlier this month, most of the GEMM Lab and I attended the 25th Biennial Conference on the Biology of Marine Mammals in Perth, Western Australia. This year’s theme, “Fishing for Change,” acknowledged that incidental entanglement in fishing gear is currently the most pervasive threat to marine mammals (e.g., Avila et al., 2018). While many presentations on the prevalence and impacts of entanglement on marine mammals were sobering, it was also inspiring to be surrounded by so many dedicated people working to address this urgent issue. For me, one of the most memorable anecdotes was an incredible whale disentanglement story shared by Paul Cottrell, a Marine Mammal Coordinator at the Department of Fisheries and Oceans Canada (DFO) in British Columbia.

An Incredible Story of Whale Disentanglement

During August 2024, DFO and a local NGO (Straitwatch) responded to a report of two humpback whales entangled in the same fishing gear near Quadra Island, B.C., Canada. Their photo-identification histories revealed that one whale had migrated from Hawaii, while the other had come from Mexico. Now tied together, the two whales’ fates became intertwined, forcing them to coordinate their movements. This situation obviously raised concerns about their welfare and survival, but I also had to silently wonder, “Did the two whales ever argue about where to migrate next? Would they choose Hawaii or Mexico?”

Thanks to the rescuers’ efforts, both whales were freed and able to make their own choice about where to spend the breeding season. As Paul explained, successfully disentangling one whale is challenging and dangerous, so freeing two was an impressive feat. After the rescue, a video showed the whales continuing to swim together synchronously, as if they did not realize they were no longer connected!

Most Entangled Whales are Out of Sight

The story above exemplifies a “confirmed” entanglement—these whales were seen dragging fishing gear and the event was reported by concerned citizens. However, most entanglement events are never witnessed, for several reasons.

When a whale becomes entangled in fishing gear, it rarely remains anchored in place. Instead, the whale often breaks part of the gear, dragging it behind as it swims. The likelihood of observing the entangled whale subsequently depends on both the chance of it being seen and the observer’s awareness and willingness to report the event (Robbins and Mattila, 2004).

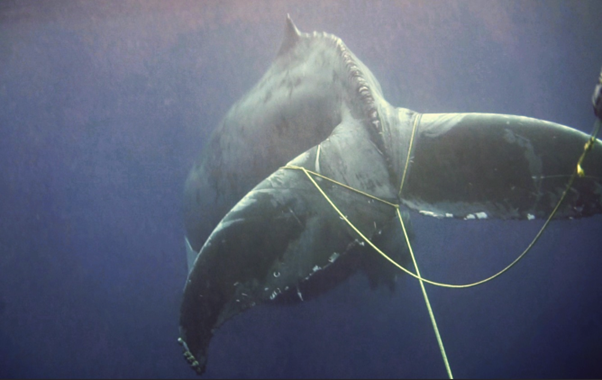
An entangled humpback whale drags gear off of San Diego, California. Credit: Keith Yip, taken under NOAA Permit #18786.

Once entangled, many become a “dead whale swimming,” eventually succumbing to starvation and/or infections (Dolman and Moore, 2017). Many entanglements involve the mouth, severely impacting the whale’s ability to feed (Moore and van der Hoop, 2012). The additional drag imposed by entanglement is comparable to the energetic costs of migration or reproduction, causing a significant depletion in their energy reserves (van der Hoop et al. 2015). Serious injuries include amputations, hemorrhage, and infections (Cassoff et al., 2011).

Although some carcasses of entangled whales wash ashore, most are lost at sea and never recovered. For example, even with relatively intensive monitoring for North Atlantic right whale (NARW) carcasses, Pace et al. (2021) estimated that recovered carcasses represented just 36% of the total deaths. These recovered carcasses may also underestimate the toll of entanglement; entanglement accounted for 51% of mortality in the carcasses vs. 87% of serious injuries observed in living NARWs (Pace et al., 2021).

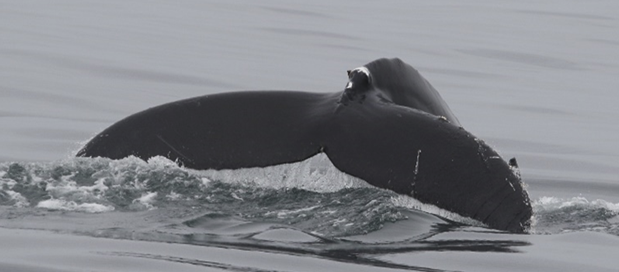
For whales that manage to dislodge the gear and survive, scars can provide clues to their past entanglement history. Injuries from the fishing lines can leave indentations where they cut through skin and blubber, and healed wounds often result in white pigmented scars that wrap around the body (especially the flukes and peduncle; e.g., Robbins and Matilla 2004). The widespread prevalence of these scars suggests that in many cases, whales can actually dislodge the gear on their own. For example, a study of entanglement scars on humpback whales in the Gulf of Maine revealed that 10% of adults and 30% of juveniles acquired new entanglement scars between 2009-2010. Without scarring analyses though, most of these entanglements would have been missed; just 7% of these individuals with entanglement-related scars were seen while entangled (Robbins 2012).

A humpback whale fluke and peduncle showing scarring likely caused by a past entanglement. Credit: GEMM lab, taken under NOAA Permit # 27426 issued to MMI.

Unfortunately, scars are not the only long-term consequence of non-lethal entanglement events. Previously entangled NARWs have lower survival rates than unaffected individuals (Robbins et al. 2015, Reed et al. 2024), and long-term stress responses can impact their future health and reproductive success (Pettis et al. 2004). It is tempting to assume that only severe entanglements affect future reproduction and survival, but a lack of extensive external injuries doesn’t necessarily mean that the impact of the entanglement event is more minor (Robbins and Matilla, 2004). For example, Reed et al. (2024) found that NARWs with entanglement injuries classified as minor were less likely to transition from a “non-breeder” to “breeder” status than those with severe injuries.

Tracking Unseen Entanglements: Project SLATE

Since reported entanglements and recovered carcasses reveal just a fraction of actual entanglements, researchers are continuing to innovate ways of documenting these “unseen” entanglement events.

As discussed in a previous blog post, photos of entanglement scars on the flukes and peduncles of humpback whales are being utilized in Project SLATE to detect trends in entanglement off the coast of Oregon, USA. Analyzing images of whales for signs of past entanglements is a meticulous process that may not seem as thrilling as responding to an actual disentanglement event. However, in areas with lower population densities, such as the Oregon coast, reported entanglements are undoubtedly an underestimate of the true number of events. Thus, tracking scarring rates can provide more comprehensive data on entanglement prevalence in Oregon than confirmed reports alone.

What to do if you see an entangled whale

If you happen to observe an entangled whale, please do not attempt to disentangle it yourself. Whale disentanglement is dangerous and complex, so best left to the experts! When well-meaning citizens attempt a disentanglement on their own, it can also result in an “incomplete disentanglement,” where some, but not all, gear is removed from the whale. Incomplete disentanglements just make it harder for responders to subsequently find and successfully rescue the whale.

Instead, report the entanglement by promptly calling:

  • Entanglement Reporting Hotline: 1-877-SOS-WHAL or 1-877-767-9425
  • or U.S. Coast Guard: VHF Ch. 16

Videos or photos showing the entangling gear is very helpful to trained responders, but remember to stay at least 100 yards from the whale, and beware of snagging your vessel in the lines. Visit NOAA Fisheries for more information.  

A NOAA-led team disentangle a humpback whale near Dutch Harbor, Alaska. Credit: Andy Dietrick/NOAA, taken under NOAA Permit #18786.
Loading


References:

Avila, I.C., Kaschner, K., Dormann, C.F.. (2018). Current global risks to marine mammals: Taking stock of the threats. Biol. Conserv. 221, 44–58.

Cassoff, R.M., Moore, K.M., McLellan, W.A., Barco, S.G., Rotstein, D.S., Moore, M.J. (2011). Lethal entanglement in baleen whales. Dis. Aquat. Organ. 96, 175–185.

Dolman, Sarah J., and Michael J. Moore. (2024). Chapter 4: Welfare implications of cetacean bycatch and entanglements. In A. Butterworth (Ed.) Marine Mammal Welfare: Human Induced Change in the Marine Environment and Its Impacts on Marine Mammal Welfare (pp. 41-65).

Moore, M. J., and van der Hoop, J. M. (2012). The painful side of trap and fixed net fisheries: chronic entanglement of large whales. Journal of Marine Sciences, 2012.

Pace III, R. M., Williams, R., Kraus, S. D., Knowlton, A. R., & Pettis, H. M. (2021). Cryptic mortality of North Atlantic right whales. Conservation Science and Practice3(2), e346

Reed, J., New, L., Corkeron, P., Harcourt, R. (2024). Disentangling the influence of entanglement on recruitment in North Atlantic right whales. Proc. R. Soc. B Biol. Sci. 291.

Robbins, J., Mattila, D. (2004). Estimating humpback whale (Megaptera novaeangliae) entanglement rates on the basis of scar evidence. Rep. to Northeast Fish. Sci. Center, Natl. Mar. Fish. Serv. 43EANF030121 22p.

Robbins, J. (2012). Scar-Based Inference Into Gulf of Maine Humpback Whale Entanglement : 2010. Report to the Northeast Fisheries Science Center National Marine Fisheries Service, EA133F09CN0253 Item 0003AB, Task 3.

van der Hoop JM, Corkeron P, Kenney J, Landry S, Morin D, Smith J, Moore MJ. (2015). Drag from fishing gear entangling North Atlantic right whales. Mar Mamm Sci 32(2):619–642.